Phospho-p95/NBS1 (Ser343) Antibody (YA165)
(Synonyms: NBS, NBS1, P95, NBN, Nibrin, Cell cycle regulatory protein p95, Nijmegen breakage syndrome protein 1, hNbs1)
Based on 1 Customer Validation
Phospho-p95/NBS1 (Ser343) Antibody (YA165) is a Rabbit-derived and non-conjugated IgG monoclonal antibody, targeting to Phospho-p95/NBS1 (Ser343).
-
Host:
Rabbit
-
Isotype:
IgG
-
Application:
WB, ICC/IF, IHC-P, IP
-
Reactivity :
Human, Mouse
-
Formulation:
Supplied in 1*TBS (pH7.4), 0.05% BSA and 40% Glycerol. Preservative: 0.05% Sodium Azide.
-
Conjugation:
Non-conjugated


To place orders, for customer services and technical support, please contact: MedChemExpress USA
Tel: 609-228-6898 E-mail: [email protected] [email protected]




Applications
| Application |
WB

WB: Western Blot
|
ICC/IF
ICC/IF: Immunocytochemistry/
Immunofluorescence |
IHC-P
IHC-P: Immunohistochemistry-Paraffin
|
IP
IP: Immunoprecipitation
|
|---|---|---|---|---|
| Dilution Ratio | 1:500-1:1000 | 1:50-1:200 | 1:50-1:200 | Use at an assay dependent concentration. |


Product Details
Phospho-p95/NBS1 (Ser343) Antibody (YA165) is a Rabbit-derived and non-conjugated IgG monoclonal antibody, targeting to Phospho-p95/NBS1 (Ser343).
-
Host Rabbit

-
Clonality Recombinant,Monoclonal

-
Species ReactivityHuman, Mouse
-
Observed Molecular WeightObserved band size: 95 kDa
Note: Due to possible protein modifications or aggregation, the molecular weight should be confirmed by actual measurement, and the predicted value is for reference only.

-
Calculated Molecular Weight Predicted band size: 85 kDa

Synthetic phosphopeptide corresponding to residues surrounding Ser343 of Human p95/NBS1.AA range:321-370.
Endogenous
Protein A affinity purified.
Non-conjugated
Phosphorylated
IgG


Product Properties
-
Appearance
Solution
-
Formulation
Supplied in 1*TBS (pH7.4), 0.05% BSA and 40% Glycerol. Preservative: 0.05% Sodium Azide.
-
Concentration
Batch-dependent, Please check the COA for the concentration of each lot. Check Lot Concentration
-
Storage & Stability
Stored at -20°C for 1 year. Avoid repeated freeze / thaw cycles.
-
Shipping
Shipping with blue ice.


Verification Images
-
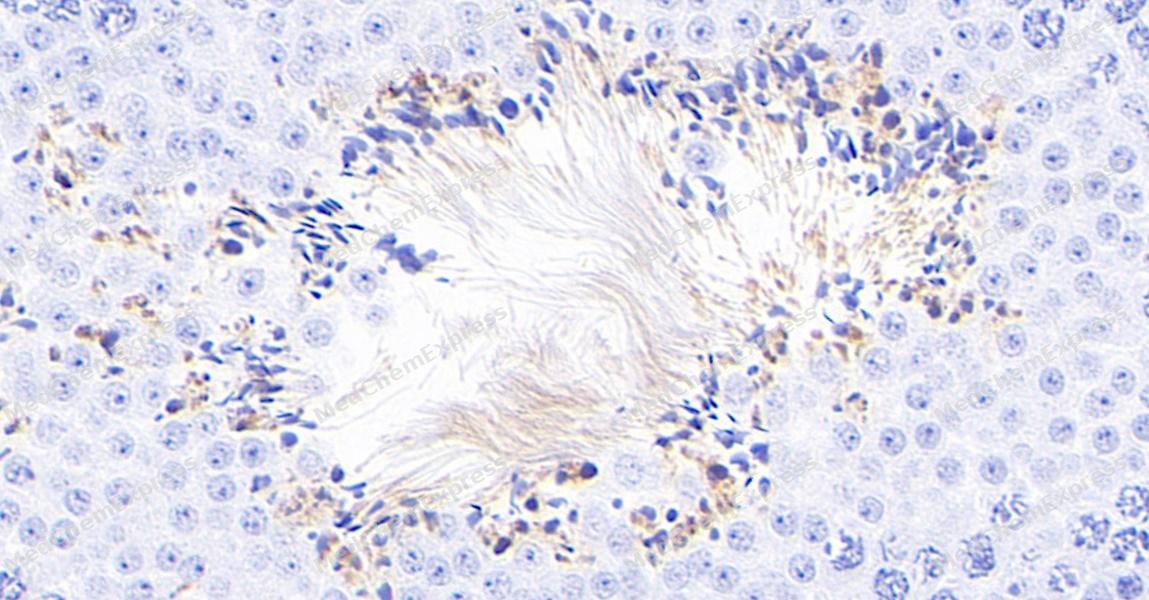 Immunohistochemical analysis of paraffin-embedded mouse testis tissue using Phospho-p95/NBS1 (Ser343) Antibody. The section was pre-treated using heat mediated antigen retrieval with Tris-EDTA buffer (pH 8.0) for 8 minutes. The tissues were blocked in QuickBlock for 20 minutes at room temperature, washed with ddH2O and PBS, and then probed with the primary antibody (HY-P80473, 1:100) in 4℃ overnight. The detection was performed using an HRP conjugated compact polymer system. DAB was used as the chromogen. Tissues were counterstained with hematoxylin and mounted with DPX.
-
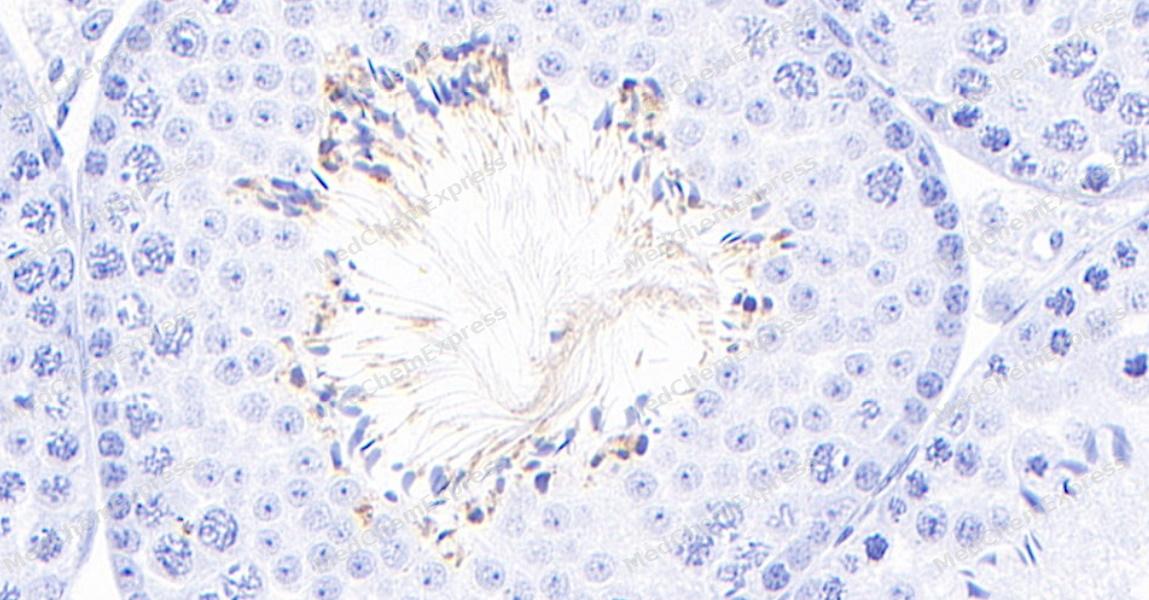 Immunohistochemical analysis of paraffin-embedded mouse testis tissue using Phospho-p95/NBS1 (Ser343) Antibody. The section was pre-treated using heat mediated antigen retrieval with Tris-EDTA buffer (pH 8.0) for 8 minutes. The tissues were blocked in QuickBlock for 20 minutes at room temperature, washed with ddH2O and PBS, and then probed with the primary antibody (HY-P80473, 1:100) in 4℃ overnight. The detection was performed using an HRP conjugated compact polymer system. DAB was used as the chromogen. Tissues were counterstained with hematoxylin and mounted with DPX.


Background
-
Function
p95/NBS1 component of the MRN complex, which plays a central role in double-strand break (DSB) repair, DNA recombination, maintenance of telomere integrity and meiosis. The MRN complex is involved in the repair of DNA double-strand breaks (DSBs) via homologous recombination (HR), an error-free mechanism which primarily occurs during S and G2 phases. The complex (1) mediates the end resection of damaged DNA, which generates proper single-stranded DNA, a key initial steps in HR, and is (2) required for the recruitment of other repair factors and efficient activation of ATM and ATR upon DNA damage. The MRN complex possesses single-strand endonuclease activity and double-strand-specific 3'-5' exonuclease activity, which are provided by MRE11, to initiate end resection, which is required for single-strand invasion and recombination. Within the MRN complex, NBN acts as a protein-protein adapter, which specifically recognizes and binds phosphorylated proteins, promoting their recruitment to DNA damage sites. Recruits MRE11 and RAD50 components of the MRN complex to DSBs in response to DNA damage. Promotes the recruitment of PI3/PI4-kinase family members ATM, ATR, and probably DNA-PKcs to the DNA damage sites, activating their functions. Mediates the recruitment of phosphorylated RBBP8/CtIP to DSBs, leading to cooperation between the MRN complex and RBBP8/CtIP to initiate end resection. RBBP8/CtIP specifically promotes the endonuclease activity of the MRN complex to clear DNA ends containing protein adducts. The MRN complex is also required for the processing of R-loops. NBN also functions in telomere length maintenance via its interaction with TERF2: interaction with TERF2 during G1 phase preventing recruitment of DCLRE1B/Apollo to telomeres. NBN also promotes DNA repair choice at dysfunctional telomeres: NBN phosphorylation by CDK2 promotes non-homologous end joining repair at telomeres, while unphosphorylated NBN promotes microhomology-mediated end-joining (MMEJ) repair. Enhances AKT1 phosphorylation possibly by association with the mTORC2 complex[1][2][3][4][5][6][7][8][9][10][11][12][13][14][15][16][17][18][19][20][21][22][23][24][25][26][27].
-
Subcellular Localization
Nucleus; Chromosome; Nucleus, PML body; Chromosome, telomere
-
Expression
Tissue_specificity:It is widely present (PubMed: 9590180) . It is highly expressed in the testes (PubMed: 9590180) .
Induction:Up-regulated by ionizing radiation (IR) -
Subunit
Component of the MRN complex composed of two heterodimers RAD50 and MRE11 associated with a single NBN (PubMed:11238951, PubMed:26215093, PubMed:28867292, PubMed:36577401, PubMed:9590181, PubMed:9705271).
-
SwissProt ID
-
Synonyms
NBS, NBS1, P95, NBN, Nibrin, Cell cycle regulatory protein p95, Nijmegen breakage syndrome protein 1, hNbs1
-
Research Field
Epigenetics and Nuclear Signaling


Documentation
-
Data Sheet (267 KB)
-
SDS (252 KB)
- English - EN (252 KB)
- Français - FR (252 KB)
- Deutsch - DE (252 KB)
- Norwegian - NO (252 KB)
- Español - ES (252 KB)
- Swedish - SV (252 KB)
- Italian - IT (252 KB)
- Korean - KR (252 KB)
- Portuguese - PT (252 KB)
-
User Guide for Antibodies (1077 KB)
References
[1]. Zhu XD, et al. Cell-cycle-regulated association of RAD50/MRE11/NBS1 with TRF2 and human telomeres. Nat Genet. 2000 Jul;25(3):347-52. [Content Brief]
[2]. Stiff T, et al. Nbs1 is required for ATR-dependent phosphorylation events. EMBO J. 2005 Jan 12;24(1):199-208. [Content Brief]
[3]. Melander F, et al. Phosphorylation of SDT repeats in the MDC1 N terminus triggers retention of NBS1 at the DNA damage-modified chromatin. J Cell Biol. 2008 Apr 21;181(2):213-26. [Content Brief]
[4]. Chapman JR, et al. Phospho-dependent interactions between NBS1 and MDC1 mediate chromatin retention of the MRN complex at sites of DNA damage. EMBO Rep. 2008 Aug;9(8):795-801. [Content Brief]
[5]. Wu L, et al. MDC1 regulates intra-S-phase checkpoint by targeting NBS1 to DNA double-strand breaks. Proc Natl Acad Sci U S A. 2008 Aug 12;105(32):11200-5. [Content Brief]
[6]. Yuan J, et al. N terminus of CtIP is critical for homologous recombination-mediated double-strand break repair. J Biol Chem. 2009 Nov 13;284(46):31746-52. [Content Brief]
[7]. Lu CS, et al. The RING finger protein RNF8 ubiquitinates Nbs1 to promote DNA double-strand break repair by homologous recombination. J Biol Chem. 2012 Dec 21;287(52):43984-94. [Content Brief]
[8]. Rai R, et al. NBS1 Phosphorylation Status Dictates Repair Choice of Dysfunctional Telomeres. Mol Cell. 2017 Mar 2;65(5):801-817.e4. [Content Brief]
[9]. Myler LR, et al. Single-Molecule Imaging Reveals How Mre11-Rad50-Nbs1 Initiates DNA Break Repair. Mol Cell. 2017 Sep 7;67(5):891-898.e4. [Content Brief]
[10]. Trujillo KM, et al. Nuclease activities in a complex of human recombination and DNA repair factors Rad50, Mre11, and p95. J Biol Chem. 1998 Aug 21;273(34):21447-50. [Content Brief]
[11]. Kobayashi J, et al. NBS1 localizes to gamma-H2AX foci through interaction with the FHA/BRCT domain. Curr Biol. 2002 Oct 29;12(21):1846-51. [Content Brief]
[12]. Xu C, et al. Structure of a second BRCT domain identified in the nijmegen breakage syndrome protein Nbs1 and its function in an MDC1-dependent localization of Nbs1 to DNA damage sites. J Mol Biol. 2008 Aug 29;381(2):361-72. [Content Brief]
[13]. Lloyd J, et al. A supramodular FHA/BRCT-repeat architecture mediates Nbs1 adaptor function in response to DNA damage. Cell. 2009 Oct 2;139(1):100-11. [Content Brief]
[14]. Wang JQ, et al. Interaction between NBS1 and the mTOR/Rictor/SIN1 complex through specific domains. PLoS One. 2013;8(6):e65586. [Content Brief]
[15]. Wang Q, et al. Rad17 recruits the MRE11-RAD50-NBS1 complex to regulate the cellular response to DNA double-strand breaks. EMBO J. 2014 Apr 16;33(8):862-77. [Content Brief]
[16]. Deshpande RA, et al. Nbs1 Converts the Human Mre11/Rad50 Nuclease Complex into an Endo/Exonuclease Machine Specific for Protein-DNA Adducts. Mol Cell. 2016 Nov 3;64(3):593-606. [Content Brief]
[17]. Anand R, et al. Phosphorylated CtIP Functions as a Co-factor of the MRE11-RAD50-NBS1 Endonuclease in DNA End Resection. Mol Cell. 2016 Dec 1;64(5):940-950. [Content Brief]
[18]. Zdravković A, et al. A conserved Ctp1/CtIP C-terminal peptide stimulates Mre11 endonuclease activity. Proc Natl Acad Sci U S A. 2021 Mar 16;118(11):. [Content Brief]
[19]. Ikura M, et al. Acetylation of Histone H2AX at Lys 5 by the TIP60 Histone Acetyltransferase Complex Is Essential for the Dynamic Binding of NBS1 to Damaged Chromatin. Mol Cell Biol. 2015 Dec;35(24):4147-57. [Content Brief]
[20]. Lee JH, et al. Direct activation of the ATM protein kinase by the Mre11/Rad50/Nbs1 complex. Science. 2004 Apr 2;304(5667):93-6. [Content Brief]
[21]. Lee JH, et al. ATM activation by DNA double-strand breaks through the Mre11-Rad50-Nbs1 complex. Science. 2005 Apr 22;308(5721):551-4. [Content Brief]
[22]. Dupré A, et al. Two-step activation of ATM by DNA and the Mre11-Rad50-Nbs1 complex. Nat Struct Mol Biol. 2006 May;13(5):451-7. [Content Brief]
[23]. Wu J, et al. Skp2 E3 ligase integrates ATM activation and homologous recombination repair by ubiquitinating NBS1. Mol Cell. 2012 May 11;46(3):351-61. [Content Brief]
[24]. Ha GH, et al. Pellino1 regulates reversible ATM activation via NBS1 ubiquitination at DNA double-strand breaks. Nat Commun. 2019 Apr 5;10(1):1577. [Content Brief]
[25]. Warren C, et al. Structure of the human ATM kinase and mechanism of Nbs1 binding. Elife. 2022 Jan 25;11:. [Content Brief]
[26]. Anand R, et al. NBS1 promotes the endonuclease activity of the MRE11-RAD50 complex by sensing CtIP phosphorylation. EMBO J. 2019 Apr 1;38(7):. [Content Brief]
[27]. Chang EY, et al. MRE11-RAD50-NBS1 promotes Fanconi Anemia R-loop suppression at transcription-replication conflicts. Nat Commun. 2019 Sep 19;10(1):4265. [Content Brief]

 Powered by Bioz