



 LinkedIn
 Researchgate
 Instagram
 X
 Facebook
 WhatsApp
 Reddit
 Mail
SARS-CoV-2 contains four main structural proteins: spike (S), membrane (M), envelope (E), and nucleocapsid (N) proteins. All the proteins and subcellular structures of CoVs are promising targets for SARS-CoV-2 research.
Articles
All
-
All
-
Scientific Reviews
-
EDM
-
Blog
Most Recent
-
Most Recent
-
Oldest
-
 Scientific Reviews
-
 Scientific Reviews
The concept of ADC can be traced back to the early 1900s, It is a visionary magic bullet that could deliver a toxic drug to certain malignant cells without affecting other normal tissues. Now, it seems that a golden age of ADC drug development is coming.
-
 Scientific Reviews
It's has been proved that p53, as a tumor suppressor gene and immune guardian, may become a destroyer through its own mutation. Moreover, the mechanism of p53 was found to be related to ferroptosis. This article mainly explores the mechanism between p53 and ferroptosis in detail.
-
 Scientific Reviews
TME (Tumor microenvironment) is considered as a complex integrated system, composed of cellular components such as tumor cells and immune cells, as well as non-cellular components such as ECM and cytokines. According to the spatial distribution of immune cells in TME, "hot" and "cold" TME will be explained in this article.
-
 Scientific Reviews
Necroptosis, also known as necroptosis, is a form of regulated necrotizing cell death mediated by RIP1 and RIP3 kinases. Necroptosis is a process that prevents the self-destruction of activated cells that are blocked by apoptosis. Necroptosis plays a tumor suppressor role in most cases. It may provide benefits in the researches of a variety of human diseases involving immune inflammation and cell death.
-
 Scientific Reviews
HLA-E, A Novel Immune Checkpoint
2023-06-29
Immune checkpoints have immunosuppressive functions. It can be used in the research of tumor immunotherapy. In this article, we introduce a new paper entitled "Immune checkpoint HLA-E: CD94 - NKG2Amediates evasion of circulating tumor cells from NK cell surveillance "research paper. -
 Scientific Reviews
WHO's Q2 drug list has been updated. Let's take you through the list of the most noteworthy small molecule drugs that we should pay attention to.
-
 Scientific Reviews
FDA Approved Drug List!
2023-09-14
In the first half of 2023 (as of June 27), the FDA approved 26 new drugs, let's take you learn about it through the article. -
 Scientific Reviews
IHC is an indispensable technique for studying tissue morphology and in situ antigen expression, but usually only one or two antigens in tissues can be stained for analysis. It cannot judge the results more intuitively. Today, Little M will introduce you to the upgraded version mlHC.
-
 Scientific Reviews
A suitable model is crucial in drug screening experiments. Organs can mimic the three-dimensional functional structure of internal organs, have similar spatial organization to corresponding organs, maintain some key characteristics, and reproduce some physiological functions. They are widely used for modeling and personalized drug screening of diseases such as cancer, infectious diseases, and rare diseases.
-
 Scientific Reviews
FDA Annual Review | Record-breaking number of new drug approvals in 2023!
-
 Scientific Reviews
KRAS, a gene we've heard so much about, has quickly risen to fame after shedding its "undruggable" label. After reading numerous articles, it's easy to feel overwhelmed and wonder: What exactly should we know about this often-discussed but previously "undruggable" target KRAS?
-
 Scientific Reviews
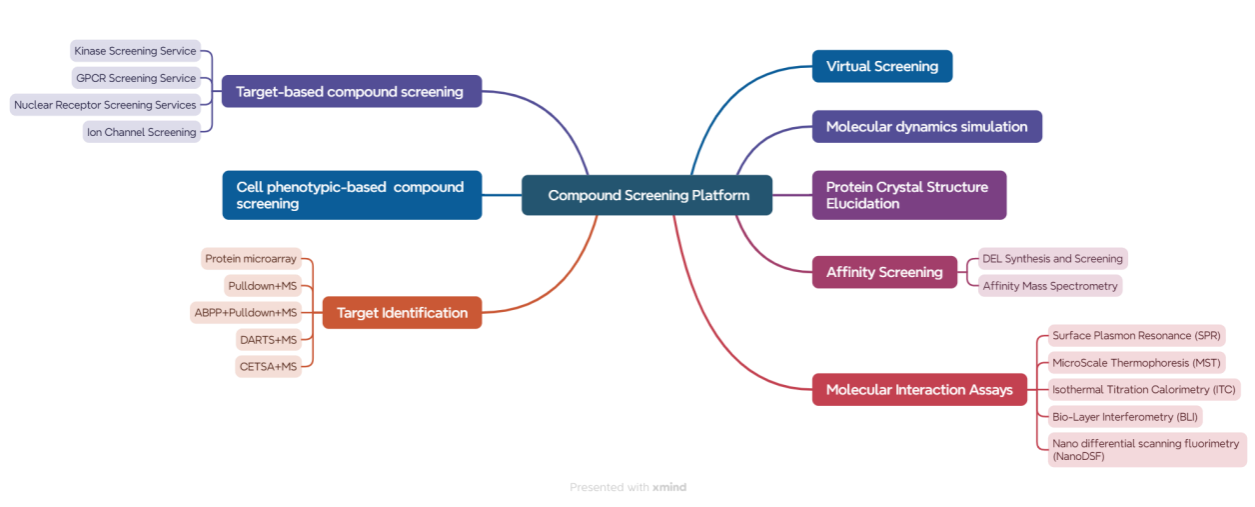
Compound Screening Guide!
2024-03-15
How to use compound library? How to design an experiment if you buy a compound library? Want a specific experimental protocol? This article will introduce popular experimental techniques and provide new ideas for publishing high level literature. -
 Scientific Reviews
Wnt/β-catenin and tumor EMT
2024-03-18
Epithelial-Mesenchymal Transition (EMT) is closely related to the plasticity of tumor cells and is a necessary process for tumor metastasis. Wnt/β-catenin is one of the main actors involved in the EMT process. Today, we’re here to popularize the tumor EMT and Wnt/β-catenin pathway~ -
 Scientific Reviews
The 2024 AACR meeting concluded successfully in California, USA. Which antitumor drugs stole the show at this conference?
-
 Scientific Reviews
Katalin Karikó and Drew Weissman were awarded the Nobel Prize in Physiology or Medicine in 2023 for their groundbreaking work in nucleoside modification, which paved the way for the creation of successful mRNA vaccines to fight against COVID-19. Let's now delve into the complete process of mRNA vaccine development.
-
 Scientific Reviews
Exosomes, which won the Nobel Prize in 2013, are still a research hotspot in the national natural sciences, and their popularity has only increased over the past decade (in 2022, they still rank 5th in the national natural sciences hotspots!). Why have exosomes become the darling of scientific research? Let's take a look together~
-
 Scientific Reviews
How important is the compound library? It connects to drug screening on one end and leads to lead compound modifications on the other, serving as one of the sources of new drug development.
-
 Scientific Reviews
Antibodies!
2024-07-26
Today, We introduce antibodies for everyone! -
 Scientific Reviews
What Are Popular Anti-tumor Drug Targets?
2024-08-20
The rapid development of targeted anti-cancer drugs has spurred diverse research across various modalities. These include small molecules, monoclonal antibodies (mAbs), cell immunotherapies, antibody-drug conjugates (ADCs), and PROTACs (proteolysis targeting chimeras). -
 Scientific Reviews
Virtual Screening and New Uses for Old Drugs
2024-09-17
With the advancement of medical science, drug screening against various disease targets has become the fundamental strategy for drug development. Currently, computer-based virtual screening techniques are emerging in the field of new drug research due to their efficiency and low cost. Let's explore it today! -
 Scientific Reviews
2024 Nobel Prize Announcements! Curious about the details? Click to dive into the exciting developments!
-
 Scientific Reviews
We are thrilled to share the latest advancements in AI technology as highlighted in this insightful article. From groundbreaking innovations to transformative applications, the future of AI is brighter than ever!
-
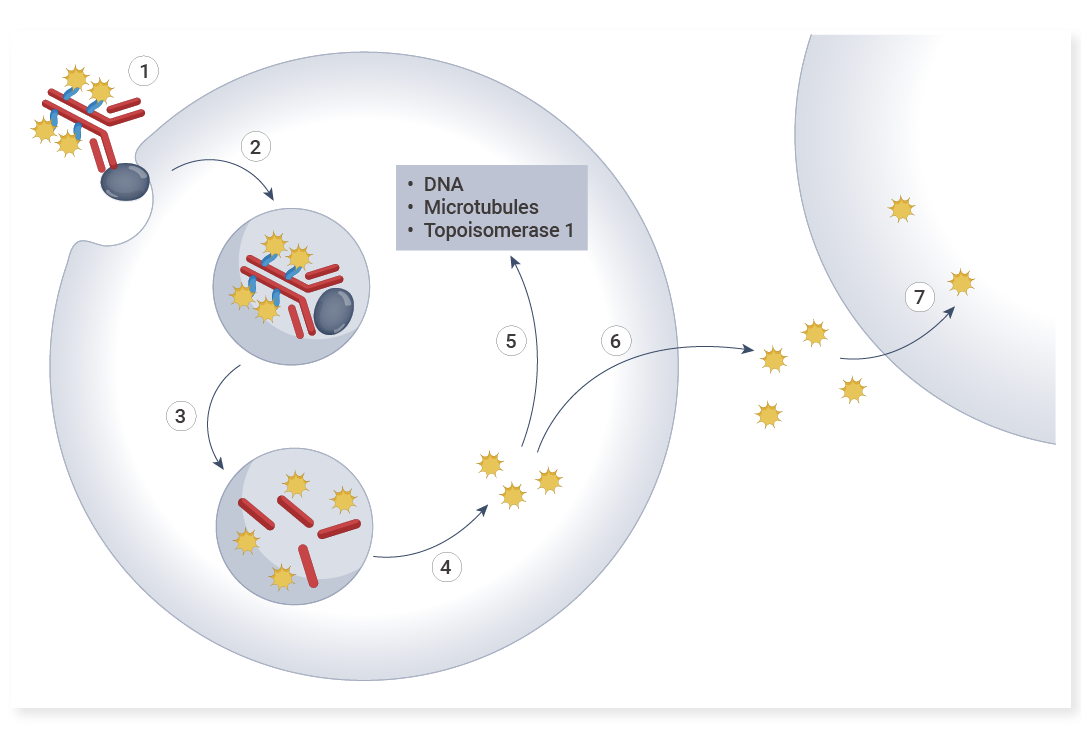 Scientific Reviews
This article will walk you through the remarkable impacts of anti-payload antibodies, delving into how these molecules are revolutionizing drug development and biological research!
-
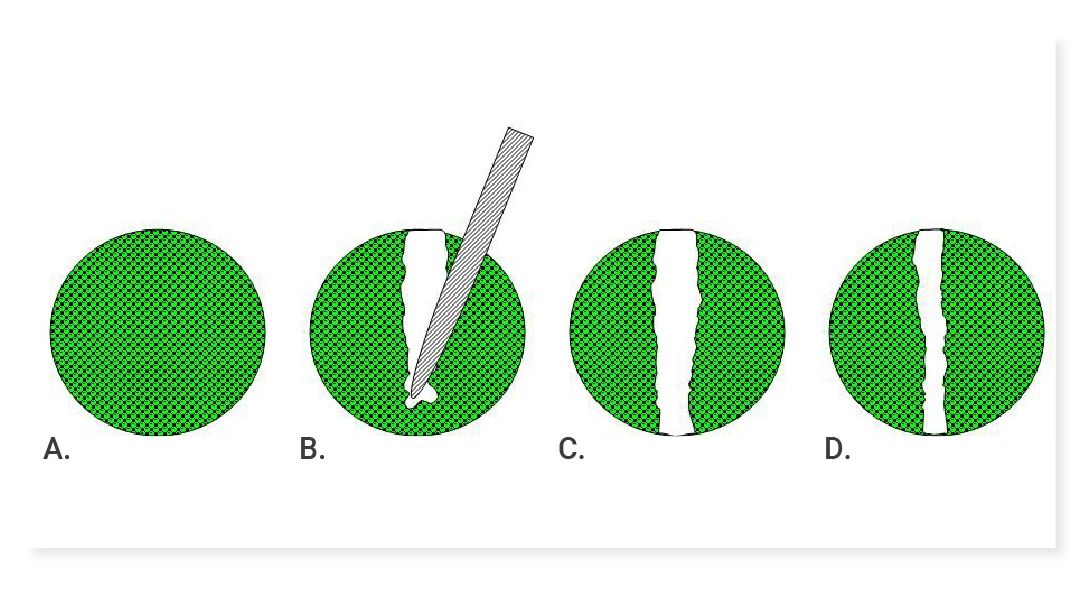 Scientific Reviews
Cell Migration vs. Invasion: Differences Revealed by Scratch Assays and Transwell Experiments
2025-05-30
In scientific research, cell migration and invasion are crucial for understanding many important biological processes. This article delves into commonly used detection methods: the scratch assay and Transwell migration/invasion assay. -
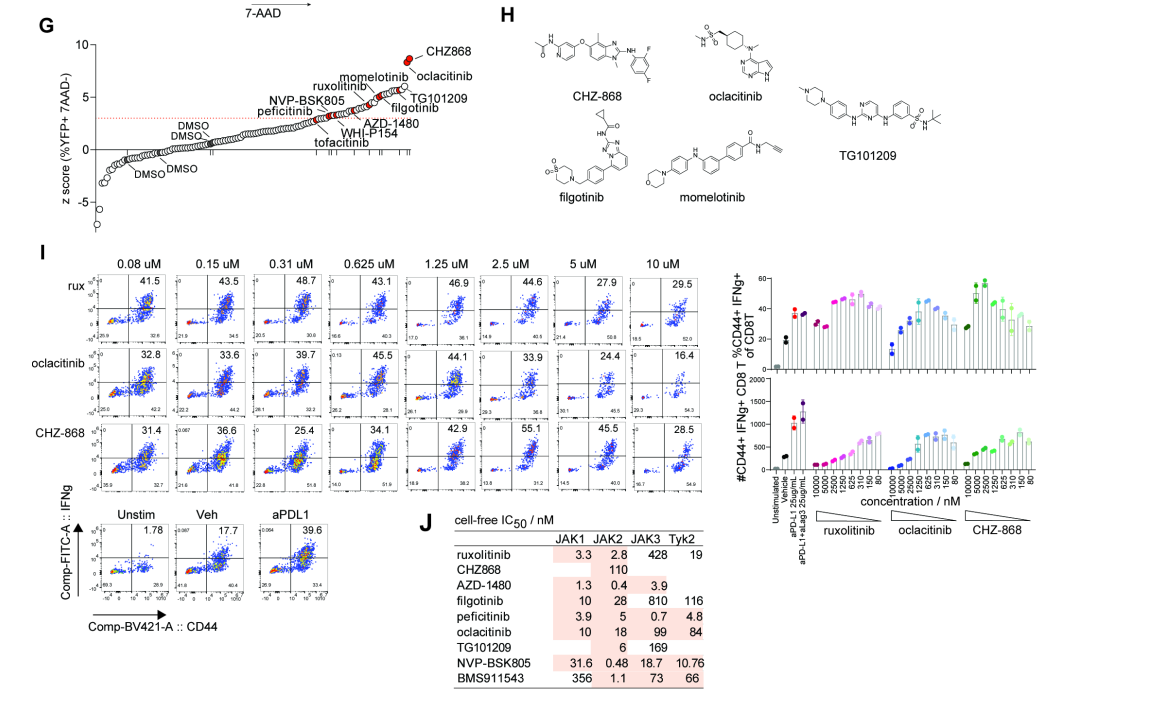
 Scientific Reviews
How should drug screening experiments be conducted? How can we ensure the accuracy of the lead compounds identified? This article will take you through how MCE's clients conduct drug screening experiments.
-
 Scientific Reviews
In this issue, we will conduct an in-depth interpretation from the dimensions of nanoparticle design, mechanism of action, in vivo and in vitro efficacy, and immune regulation, revealing how this research brings new hope for the treatment of invasive tumors through interdisciplinary innovation!
-
 Scientific Reviews
IHC, ICC, IF Techniques: A Practical Guide
2025-07-25
Confused About IHC/ICC/IF? Why Does Immunostaining Seem So Complicated? Read This Now! Master Immunostaining with Confidence! -
 Scientific Reviews
HTS Breakthroughs Powered by MCE Libraries
2025-08-13
Key High-Throughput Screening Breakthroughs of 2024 Featuring MCE -
 Scientific Reviews
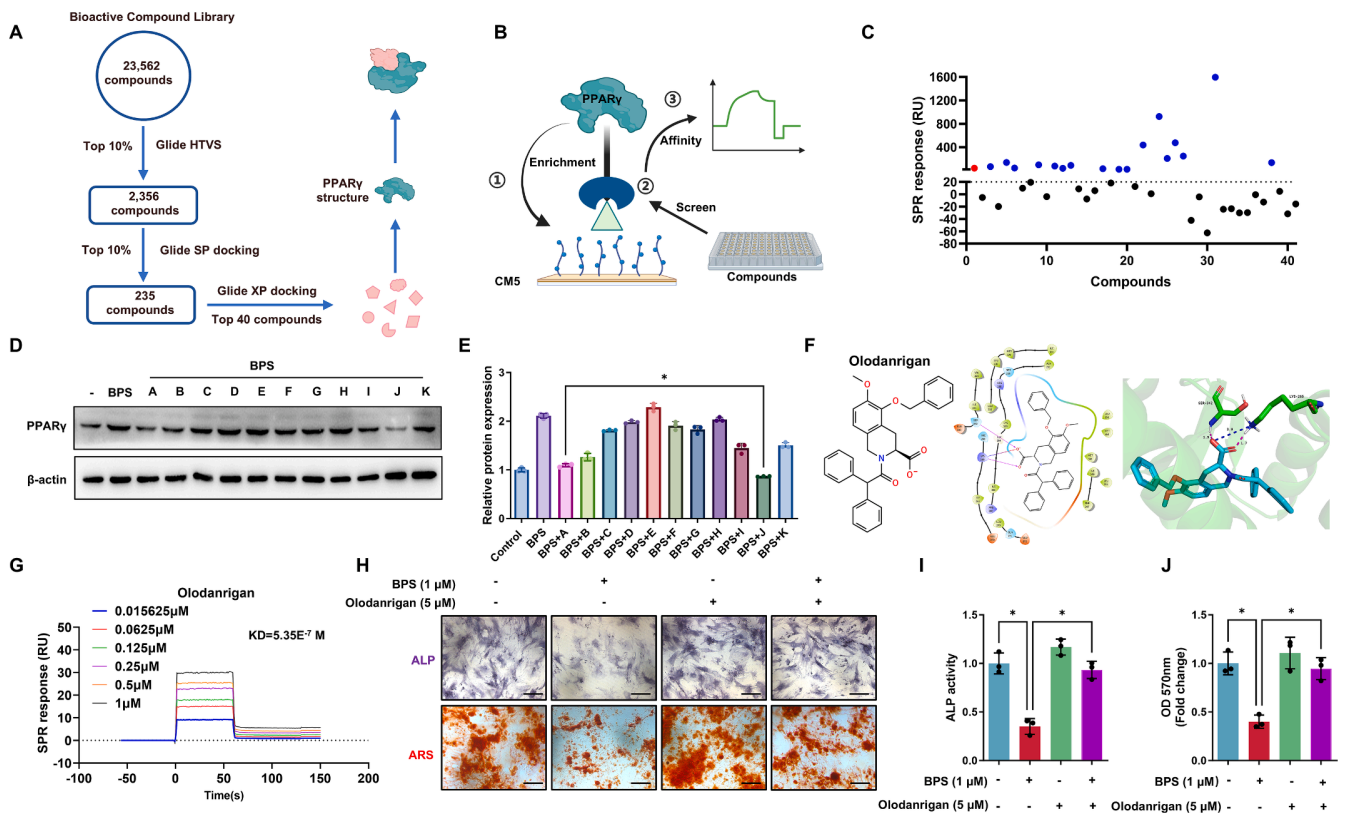
Encountering challenges with the high costs and long timelines of drug screening? Have a defined target but remain uncertain how to efficiently identify active molecules? Unsure how to validate hits generated from virtual screening? The ‘Winning Combination’ of drug screening offers a powerful solution to address these critical obstacles.
-
 Scientific Reviews
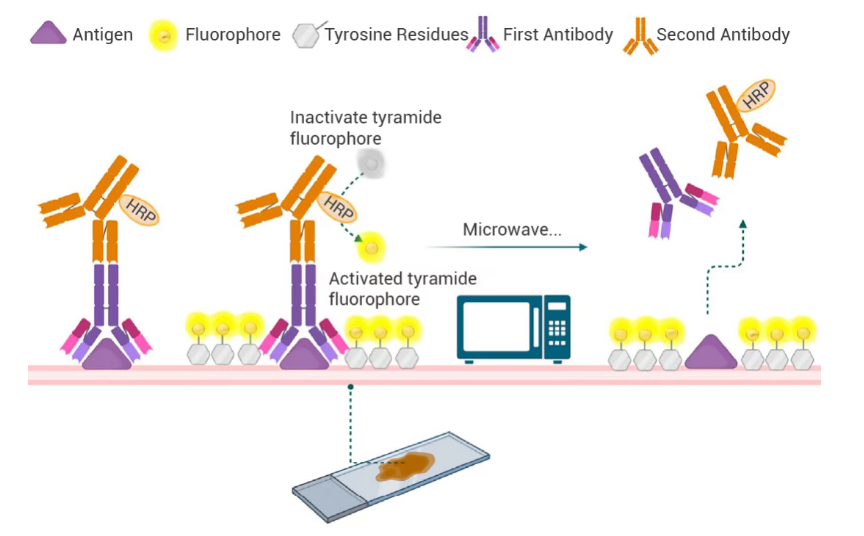
This detailed guide outlines the standardized experimental protocols for multiplex immunohistochemistry (mIHC), systematically summarizes common technical issues encountered during sample preparation, staining and imaging processes, and provides practical troubleshooting solutions to ensure reliable and reproducible results in biomedical research and clinical sample analysis.
-
 Scientific Reviews
Exosomes—natural nanoscale carriers—are revolutionizing targeted therapy. This article uncovers the science behind their precision in drug delivery.
-
Scientific Reviews
Cracking the PROTAC Permeability Barrier: CD36-Mediated Endocytosis as a Potential Breakthrough2025-12-03
This article provides an in-depth analysis of cutting-edge literature revealing CD36 as a key mediator of cellular uptake for PROTACs and bRO5 compounds. By structurally optimizing PROTAC molecules to enhance their affinity for CD36, membrane permeability can be markedly improved, leading to significantly enhanced antitumor efficacy. -
 Scientific Reviews
This paper elaborates on cytokines for culturing major immune cells, their regulatory roles, recombinant cytokines' merits and MCE’s related high-quality products.
-
 Scientific Reviews
This article walks you through the experimental design and workflow of flow cytometry, delivering a clear, dynamic, and professional overview to elevate your research.
-
 Scientific Reviews
Molecular glue degraders have evolved from a serendipitous observation to one of the most dynamic and transformative fields in biomedical research.
-
 EDM
Research Solution for Breast Cancer TME
2025-05-21
This review examines the complex interactions within the breast cancer tumor microenvironment, emphasizing how understanding these dynamics is essential for developing effective therapies and overcoming immune resistance. -
 EDM
This review discusses the fundamentals of lipid biology and lipid metabolism, examines dysregulated lipid metabolism in cancer, and summarizes therapeutic strategies targeting lipid metabolic pathways.
-
 EDM
This review presents an overview of antibody–drug conjugates from design principles and antitumor mechanisms to structural innovations, clinical progress, and future development prospects.
-
 EDM
This review explores mechanisms and strategies for modulating the gut microbiota to enhance cancer immunotherapy, providing insights to improve therapeutic efficacy.
-
 EDM
Combating Immune Evasion in Cancer
2025-10-15
This review summarizes the mechanisms by which tumors evade immune surveillance and discusses therapeutic strategies to restore antitumor immunity. -
 EDM
This review summarizes the mechanisms of drug resistance in triple-negative breast cancer and highlights emerging therapeutic strategies.
-
 EDM
Bispecific Antibodies in Cancer Therapy
2025-10-29
This review highlights the mechanisms, technology platforms, and clinical progress of bispecific antibodies, and discusses emerging strategies to guide future development. -
 EDM
This review provides insights into the pancreatic ductal adenocarcinoma tumor microenvironment, highlighting its cellular composition, stromal heterogeneity, and immune-targeting strategies.
-
 EDM
Understanding In Vivo CAR-T Cell Therapy
2026-01-22
This review provides a comprehensive overview of in vivo CAR-T therapy, covering technical platforms, clinical translation, and key challenges such as gene delivery and immunogenicity. -
 EDM
Highlight single-cell metabolomics and stable isotope tracing (SIT) in uncovering metabolic heterogeneity and nutrient flux dynamics in tumors.
-
 EDM
Explore ADC evolution, immune combination strategies, and clinical advances at the intersection of targeted therapy and immunotherapy.
-
 EDM
Tumor Organoid-Immune Cell Co-Culture Models: Advances, Applications, and Future Directions
2026-05-07
Summarize technical strategies, application advances, and future directions of tumor organoid–immune co-culture systems. -
 EDM
Review mechanisms, major challenges, and efficacy-enhancing strategies of TCR-T therapy in solid tumors, with implications for future research and clinical translation.
-
 EDM
The Dual Role of Cellular Senescence in Cancer: Mechanisms, Microenvironment, and Therapeutics
2026-05-21
Explore the dual role of cellular senescence in cancer, including tumor suppression, SASP-driven tumor promotion, senescence heterogeneity and plasticity, and advances in senescence-targeted therapies. -
 EDM
Breaking Immune Resistance in Colorectal Cancer: From Molecular Mechanisms to Precision Therapy
2026-06-25
Explore CRC molecular subtypes, immune landscapes, resistance mechanisms, and emerging precision strategies for improving outcomes across distinct subtypes. -
 EDM
Explore the mechanisms of tumor immune evasion, dynamic checkpoint regulation, and the evolution of mechanism-driven combinations and patient stratification.
-
 Blog
EC0489, a SMDC for Cancer Therapy
2019-03-25
EC0489, a conjugate of folic acid and desacetyl vinblastine hydrazide, is a SMDC under development for the treatment of solid tumours. -
 Blog
R916562, a dual Axl/VEGF-R2 inhibitor, could be a potential anti-angiogenic and anti-metastatic drug for cancer chemotherapy.
-
 Blog
Role of PRMT7 Probe SGC3027 in Cancer
2019-03-27
SGC3027 is the first potent, selective and cell active chemical probe for PRMT7. SGC3027 is also a pro-drug, which converts to the active compound SGC8158 -
 Blog
Alofanib, An Allosteric Inhibitor of FGFR2
2019-03-28
Alofanib is an allosteric inhibitor of FGFR2 and inhibits FGF-mediated proliferation with GI50s of 16-370 nM, showing pronounced antitumor activity. -
 Blog
A Novel and Efficacious RAF Inhibitor RAF709
2019-03-30
RAF709, a novel and efficacious RAF inhibitor, activates the MAPK pathway and shows antitumor activity in tumor cells harboring BRAF or RAS mutations. -
 Blog
CF53 is a highly potent, selective and orally active inhibitor of BET protein, with anti-tumor activity in acute leukemia and breast cancer cell lines.
-
 Blog
AZD3229 is a Potent Pan-KIT Mutant Inhibitor
2019-04-04
AZD3229 is a potent, pan-KIT mutant inhibitor with potent single digit nM growth inhibition against a diverse panel of mutant KIT driven Ba/F3 cell lines. -
 Blog
BR351 is a Brain Penetrant MMP Inhibitor
2019-04-05
BR351 is a brain penetrant MMP inhibitor, and a potential tool for the molecular imaging of activated MMPs with PET, with an IC50 in the nanomolar range. -
 Blog
A Lead PROTAC BRD9 Chemical Degrader
2019-04-06
PROTAC BRD9 Degrader-1 is a lead PROTAC BRD9 chemical degrader and a selective probe useful for the study of BAF complex biology. -
 Blog
SGC-GAK-1 is a potent, selective, and cell-active GAK inhibitor and shows potent anti-proliferative activity in LNCaP and 22Rv1 cells.
-
 Blog
COH000 is an allosteric, covalent and irreversible inhibitor of SUMO-activating enzyme, with an IC50 of 0.2 μM for SUMOylation in vitro.
-
 Blog
MK-0429 is An Oral Integrin (αvβ3) Inhibitor
2019-04-11
MK-0429, an orally active αvβ3 inhibitor, is a potential therapeutic agent for the prevention of kidney fibrosis, melanoma and osteoporosis. -
 Blog
AZ304, a Dual BRAF Inhibitor Against Cancer
2019-04-12
AZ304 is a potent BRAF inhibitor, blocks both wild type BRAF and V600E mutant BRAF activity, with IC50s in the nanomolar range. -
 Blog
Erteberel is a Selective ERβ Agonist
2019-04-16
Erteberel (LY500307) is a synthetic, nonsteroidal estrogen which acts as a selective ERβ agonist and under development for the treatment of schizophrenia. -
 Blog
MBQ-167 is a dual Rac/Cdc42 inhibitor in in metastatic cancer, with IC50s of 103 nM for Rac 1/2/3 and 78 nM for Cdc42 in MDA-MB-231 cells, respectively.
-
 Blog
PRN1008 is a Reversible Covalent and Oral Active Inhibitor of Bruton’s Tyrosine Kinase (BTK)
2019-04-18
PRN1008 is a selective, reversible covalent and oral active inhibitor of Bruton’s Tyrosine Kinase (BTK), with an IC50 of 1.3 nM. -
 Blog
Multiple Tyrosine Kinases Inhibitor TAS-115
2019-04-19
TAS-115 is a potent VEGFR and c-Met/HGFR-targeted kinase inhibitor with IC50s of 30 and 32 nM for rVEGFR2 and rMET, respectively. -
 Blog
Y06036 is a potent and selective BET inhibitor for potential treatment of castration-resistant prostate cancer. With nanomolar inhibition.
-
 Blog
JNJ-64619178 is a selective and pseudo-irreversible PRMT5 inhibitor with an IC50 of 0.14 nM. Has potent Activity In Lung Cancer.
-
 Blog
(E)-AG 99 is an EGFR inhibitor and shows a growth-inhibition on not only serum-starved cells but also normally grown cells. Treatment for Bladder cancer.
-
 Blog
TAK-828F is a potent, selective and orally active retinoic acid receptor-related orphan receptor γt (RORγt) inverse agonist. TAK-828F inhibits IL-17A cytokine expression and reduces symptoms of autoimmune encephalomyelitis mice.
-
 Blog
Y06137 is a potent and selective BET inhibitor, which binds to the BRD4(1) bromodomain with a Kd of 81 nM. Antitumor activity.
-
 Blog
Borussertib is a covalent-allosteric and first-in-class inhibitor of protein kinase Akt, with an IC50 of 0.8 nM and a Ki of 2.2 nM for Akt-wt.
-
 Blog
NRX-252262 is a β-catenin:β-TrCP interaction enhancer, and its cognate E3 ligase, SCFβ-TrCP, induces mutant β-catenin degradation, with an EC50 of 3.8 nM
-
 Blog
TAK-981 is a selective inhibitor of the SUMOylation enzymatic cascade, with potential immune-activating and antineoplastic activities
-
 Blog
TD-428 is a Highly Specific BRD4 Degrader
2019-04-29
TD-428, a immunomodulatory drug analog, is a highly specific BRD4 degrader with a DC50 of 0.32 nM. TD-428 reduces c-Myc levels more efficiently than JQ1. -
 Blog
SLLN-15 is an oral activ enhancer of autophagy that activates cytostatic macroautophagy/autophagy in triple-negative breast cancer (TNBC).
-
 Blog
A1874 is a nutlin-based and BRD4-degrading PROTAC with a DC50 of 32 nM. Effective in inhibiting many cancer cell lines proliferation
-
 Blog
BAY-8002 is a selective and orally active inhibitor of monocarboxylate transporter 1 (MCT1), with an IC50 of 85 nM. Has potential to treat lymphoma.
-
 Blog
MRTX-1257 is a selective, irreversible, covalent and oral active KRAS G12C inhibitor, with an IC50 of 900 pM for KRAS dependent ERK phosphorylation.
-
 Blog
USL311 is a selective CXCR4 antagonist, which prevents the binding of stromal-cell derived factor-1 (SDF-1 or CXCL12) to CXCR4. Anti-tumor activity.
-
 Blog
TX1-85-1, a ATP-competitive ligand of Her3, covalent modification of Her3 to inhibit Her3 signaling
2019-06-01
TX1-85-1 is a Her3 (ErbB3) inhibitor with an IC50 of 23 nM. TX1-85-1 induces partial degradation of Her3 protein and attenuates Her3-dependent signaling. -
 Blog
IWP-O1, a Highly Potent Porcupine Inhibitor, Functions by Preventing the Secretion of Wnt Proteins
2019-06-03
IWP-O1 is a Porcupine (Porcn) inhibitor, with an EC50 of 80 pM in L-Wnt-STF cells. IWP-O1 functions by preventing the secretion of Wnt proteins[ -
 Blog
PF-06465469 is a Covalent Inhibitor of ITK
2019-06-08
PF-06465469 is a potent and covalent inhibitor of ITK with an IC50 of 2 nM. PF-06465469 inhibits MEK1/2 or AKT phosphorylation. -
 Blog
JMS-17-2 is a CX3CR1 Antagonist
2019-06-12
JMS-17-2 is a potent and selective CX3CR1 antagonist with an IC50 of 0.32 nM. Has potential to treat cancers such as breast cancer. -
 Blog
S18-000003 is a potent, selective and orally active inhibitor of retinoic acid receptor-related orphan receptor-gamma-t (RORγt). S18-000003 ameliorates psoriasis-like lesions in vivo. S18-000003 can be used for the research of skin inflammatory diseases.
-
 Blog
PTC299 is a dual and orally active DHODH and VEGF inhibitor, has broad and potent activity against hematological cancer cells.
-
 Blog
AMG 487 is an orally active and selective antagonist of CXC chemokine receptor 3 (CXCR3). AMG 487 has potential to treat metastatic cancer.
-
 Blog
FGTI-2734 is a dual farnesyl and geranylgeranyl transferase-1 inhibitor. FGTI-2734 prevents membrane localization of KRAS and mutant KRAS pancreatic tumors.
-
 Blog
BI-882370 is a potent RAF kinase inhibitor with IC50s of 0.4, 0.8, and 0.6 nM for oncogenic BRAFV600E-mutant, the WT BRAF and CRAF kinases , respectively.
-
 Blog
MSX-122 is an orally active partial antagonist of CXCR4, inhibiting CXCR4/CXCL12 actions. MSX-122 has both anti-tumor and anti-metastasis activities.
-
 Blog
ZT-12-037-01 is a ATP-competitive and specific STK19 inhibitor and inhibits oncogenic NRAS-driven melanocyte malignant transformation.
-
 Blog
PT2977 is an orally active and selective HIF-2α inhibitor with an IC50 of 9 nM. PT2977 is a potential treatment for ccRCC and VHL disease.
-
 Blog
BI-2852 is a potent KRAS inhibitor with nanomolar affinity and reduces pERK and pAKT levels in a dose-dependent manner in a KRAS mutant cell line NCI-H358.
-
 Blog
BAY-293 is a potent inhibitor of Son of Sevenless 1 (SOS1) and blocks RAS activation via disruption of the KRAS-SOS1 interaction with an IC50 of 21 nM.
-
 Blog
WZ811 is an Orally Active CXCR4 Antagonist
2019-09-07
WZ811 is an orally active, highly potent competitive antagonist of CXCR4, which inhibits chronic lymphocytic leukemia progression and tumorigenesis. -
 Blog
RU-302 is a pan-TAM inhibitor that blocks the TAM Ig1 ectodomain and the Gas6 Lg domain interaction. RU-302 blocks Gas6-inducible Axl receptor activation.
-
 Blog
BAY 61-3606 is an orally available, ATP-competitive, reversible and highly selective Syk inhibitor and sensitizes apoptosis by in breast cancer.
-
 Blog
IPR-803 is a potent inhibitor of the uPAR•uPA protein-protein interaction, and binds directly to uPAR with sub-micromolar affinity.
-
 Blog
Vorolanib is an orally active, multikinase VEGF/PDGF receptor inhibitor with antitumor activity and is expected to disrupt tumor angiogenesis.
-
 Blog
CCG-222740 is a potent and selective MRTF pathway inhibitor. It effectively reduces fibrosis in the skin and blocks melanoma metastasis.
-
 Blog
IACS-8803 is a highly potent cyclic dinucleotide stimulator of interferon genes (STING) agonist with robust systemic antitumor efficacy.
-
 Blog
AC-73 is a first specific, orally active the cluster of differentiation 147 (CD147) inhibitor and specifically disrupts CD147 dimerization.
-
 Blog
CH6953755 is a potent, orally active and selective YES1 kinase inhibitor leading to antitumor activity against YES1 Gene -amplified cancers.
-
 Blog
CA-4948 is a Selective and Orally Bioavailable IRAK4 Kinase Inhibitor for Lymphoma Treatment
2020-01-05
CA-4948 is a potent, selective and orally bioavailable IRAK4 kinase inhibitor. CA-4948 can be used for the treatment of lymphoma. -
 Blog
ADH-503 is an orally active and allosteric CD11b agonist and leads to the repolarization of tumor-associated macrophages.
-
 Blog
Balixafortide is a potent, selective peptidic CXCR4 antagonist with anti-cancer effects, and blocks β-arrestin recruitment and calcium flux.
-
 Blog
CCT365623, an Orally Active LOX Inhibitor, Supresses EGFR (pY1068) and AKT Phosphorylation
2020-04-16
CCT365623 is an orally active LOX inhibitor, suppresses EGFR (pY1068) and AKT phosphorylation driven by EGF. CCT365623 has good pharmacokinetic properties. -
 Blog
RBN-2397 is an orally active accross species NAD+ competitive inhibitor of PARP7. RBN-2397 binds to PARP7 and restores interferon (Type I) signaling.
-
 Blog
GSK143 is an orally active and highly selective spleen tyrosine kinase (SYK) inhibitor. GSK143 reduces inflammation in the intestinal muscularis in mice.
-
 Blog
EW-7195 is a potent and selective ALK5 inhibitor, and efficiently inhibits TGF-β1-induced Smad signaling, EMT and breast tumour metastasis to the lung.
-
 Blog
MSA-2 is an orally available non-nucleotide STING agonist. MSA-2 shows antitumor activity and stimulates interferon-β secretion in tumors.
-
 Blog
SP-8356, an orally active CD147inhibitor, exerts anti-breast cancer effects by inhibiting NF-κB signaling. Anti-atherosclerotic effects.
-
 Blog
CB-1158, a potent and orally bioavailable inhibitor of arginase, blocks myeloid cell-mediated immune suppression in the tumor microenvironment.
-
 Blog
SRX3207 is an orally active and first-in-class dual Syk/PI3K inhibitor. SRX3207 possesses effective anti-tumor activity in vitro and in vivo.
-
 Blog
Verucopeptin inhibits v-ATPase activity by directly targeting the v-ATPase ATP6V1G subunit but not ATP1V1B2 or ATP6V1D. Also a potent HIF-1 inhibitor.
-
 Blog
E7820, sulfonamide derivative, is a unique angiogenesis inhibitor suppressing an expression of integrin alpha2 subunit on endothelium.
-
 Blog
Cyclo(-RGDfK) is a selective inhibitor of the αvβ3 integrin. Cyclo(-RGDfK) potently targets cancer cells through binding to the cell surface αvβ3 integrin.
-
 Blog
Cilengitide is a compound targeting angiogenesis, the cornerstone of tumor growth and metastasis. ανβ3 and ανβ5 are the target of Cilengitide.
-
 Blog
Tetrac inhibits the cellular actions of thyroid hormone initiated at the hormone receptor on plasma membrane integrin alphavbeta3.
-
 Blog
ENMD-1198 is an orally active microtubule-targeting agent with antiproliferative and antiangiogenic activity.
-
 Blog
TPP-1 is a potent inhibitor of the PD-1/PD-L1 interaction. TPP-1 binds specifically to PD-L1 with a high affinity (KD=95 nM).
-
 Blog
FAPI-46 is a quinoline-based FAP-targeted radiotracer. FAPI-46 has higher tumor uptake and prolonged tumor accumulation.
-
 Blog
BMSpep-57 is a potent and competitive macrocyclic peptide inhibitor of PD-1/PD-L1 interaction. It induces high levels of IL-2.
-
 Blog
ML339 is a Selective CXCR6 Antagonist
2021-05-12
ML339 is a small molecule antagonist would block Prostate cancer cell trafficking; hence mediate a metastatic event and disease progression. -
 Blog
Sitravatinib (MGCD516) is an Orally Bioavailable RTK Inhibitor with PD-1 Blockade Activity
2021-06-03
Sitravatinib, a small molecule RTK inhibitor, shows potent anti-tumor activity in preclinical models of sarcoma. -
 Blog
Motesanib (AMG 706) is an orally active VEGFR inhibitor. Potently inhibits angiogenesis and induces regression in tumor xenografts.
-
 Blog
EMD527040 is a highly selective αvβ6 antagonist with antifibrotic activities.
-
 Blog
Inupadenant is an orally active, highly selective A2A receptor antagonist with potent anti-tumor activity.
-
 Blog
UK122 is a potent and selective urokinase-type plasminogen activator (uPA) inhibitor with anti-cancer activity.
-
 Blog
AZD4635 is a potent, selective and orally active antagonist of A2AR that reverses adenosine-mediated immune suppression.
-
 Blog
Nintedanib a potent and orally active triple vascular kinase inhibitor for VEGFR1/2/3, FGFR1/2/3 and PDGFRα/β.
-
 Blog
Axitinib is a multi-targeted tyrosine kinase inhibitor and potently inhibitor VEGFR1, VEGFR2, VEGFR3 and PDGFRβ.
-
 Blog
CL097 is a TLR7/8 agonist. CL097 induces pro-nflammatory cytokines. CL097 induces NADPH oxidase priming and efficient diabetogenic cytotoxic T lymphocyte (CTL) function in NOD mice.
-
 Blog
Indoximod, an immunometabolic adjuvant, is an orally active IDO pathway inhibitor. Indoximod acts as a Trp mimetic in regulating mTOR.
-
 Blog
Tanomastat is an orally active, non-peptidic biphenyl MMPs inhibitor, with antiangiogenic, anti-invasive and antimetastatic activities.
-
 Blog
BM213 is a selective C5aR1 agonist. It’s a useful research tool to study C5aR1 function
-
 Blog
Telatinib is an orally active inhibitor of VEGFR2, VEGFR3, PDGFα, and c-Kit.
-
 Blog
Marimastat (BB2516) is a broad spectrum and orally bioavailable inhibitor of MMPs (Matrix metalloproteinases).
-
 Blog
Gardiquimod is a TLR7/8 agonist and can inhibit HIV-1 infection.
-
 Blog
Vatalanib is an inhibitor of VEGFR2/KDR. Vatalanib induces inhibition of the angiogenic response to VEGF and PDGF.
-
 Blog
Toceranib is a selective and orally active inhibitor of RTK and has the potential for the research of canine mast cell tumors.
-
 Blog
Tiragolumab is an immune checkpoint inhibitor binding to TIGIT. Tiragolumab is effective against multiple solid malignancies.
-
 Blog
Henatinib is an orally active small-molecule multikinase inhibitor that has demonstrated broad and potent antitumor activities.
-
 Blog
KGP94 is a selective inhibitor of cathepsin L. KGP94 has antitumor activity and improves survival of bone metastases bearing mice.
-
 Blog
Certepetide is a Tumor-penetrating Enhancer via RGD Motif Interaction with Alphav-integrins
2022-09-01
Certepetide is a tumor-penetrating enhancer and has the potential for the research of metastatic pancreatic ductal adenocarcinoma. -
 Blog
BSP16 is a potent, orally active stimulator of interferon genes (STING) agonist. BSP16 has potent anti-cancer activity.
-
 Blog
Parsatuzumab (RG 7414) is a humanized monoclonal antibody, that acts as an immunomodulator, and binds to EGFL7.
-
 Blog
Serplulimab is a humanized monoclonal anti-PD-1 antibody and has the potential for the research of small cell lung cancer.
-
 Blog
ABT-510, a peptide analog of thrombospondin-1 (TSP-1), can block angiogenesis in vitro and in vivo, and slow tumor growth.
-
 Blog
Mogamulizumab is an Anti-CCR4 monoclonal antibody. It enhances antibody-dependent cellular cytotoxicity and is effective against leukemia.
-
 Blog
Bapotulimab (BAY-1905254) is an ILDR2 IgG antibody that blocks the immunosuppressive effects of ILDR2 on T-cell activation.
-
 Blog
Nanrilkefusp alfa is a selective and strong IL-15 agonist. It inhibits tumor metastasis and viability by activating natural killer (NK) cells.
-
 Blog
Urabrelimab (SRF231) is an anti-CD47 monoclonal antibody, blocking the CD47-SIRPα interaction. It has the potential to research anticancer.
-
 Blog
Efineptakin alfa (NT-17) is a Long-Acting Recombinant Human IL-7 for Glioblastoma Research
2023-02-07
Efineptakin alfa (NT-17) is a long-acting recombinant human IL-7. Efineptakin alfa can be used for glioblastoma research. -
 Blog
Pegdinetanib (BMS-844203) is a selective VEGFR-2 inhibitor with antitumor activity.
-
 Blog
Tifcemalimab, a Humanized anti-BTLA monoclonal antibody, blocks the interaction of HVEM-BTLA by binding to BTLA and activates lymphocytes.
-
 Blog
Geptanolimab (CBT-501) is a programmed death-1 (PD-1) monoclonal antibody. Geptanolimab can be used in research forsolid tumor research.
-
 Blog
Dazostinag is a STING Agonist and Can be used for Antibody-Drug Conjugates (ADCs) Synthesis
2023-03-13
Dazostinag is a STING agonist and a playload, to synthesis antibody-drug conjugates (ADCs). It has antitumor activity in vivo. -
 Blog
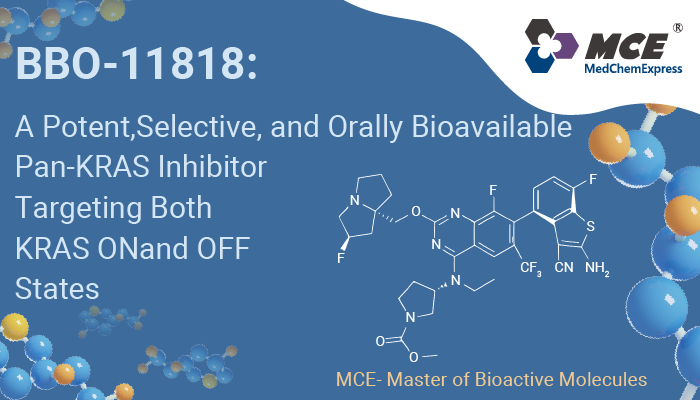
BBO-11818 is a potent, selective, orally bioavailable, and noncovalent pan-KRAS inhibitor targeting multiple clinically relevant KRAS mutants in both ON and OFF states.
Products
All
-
All
-
Inhibitors & Agonists
-
Reference Standards
-
Natural Products
Targets/Pathways
